Running Economy and 4 Proven Upgrades That Unlock Effortless Speed
Two runners with identical lung capacity can produce drastically different race results. Discover the biomechanical and cellular science of running economy and how targeted training unlocks free athletic speed.
Mastering your running economy dictates whether a sustained race pace feels like a fluid rhythm or an agonizing battle against gravity. Picture two distance runners toeing the starting line of an endurance event with identical maximum oxygen consumption values. In a physiology laboratory, their maximal aerobic power is virtually indistinguishable. On paper, both engines possess the exact same theoretical horsepower. Yet after thirty kilometers of sustained locomotion, one runner glides across the road looking relaxed and bouncy, while the other trudges along in total biomechanical collapse. That divergence does not boil down to simple mental willpower or electrolyte balance. It comes down to kinetic efficiency.
In sports physiology, running economy represents the metabolic cost of maintaining a steady submaximal velocity, quantified by the volume of oxygen or energy units consumed per kilometer. Think of it as the fuel economy rating of an automobile chassis. A vehicle equipped with an enormous fuel tank and a high-displacement engine burns through gasoline with alarming speed if its wheel alignment pulls to the left, its brake pads rub against the rotors, and its tire pressure is flat. Human locomotion operates under the exact same laws of physics. If every foot strike bleeds forward momentum into vertical bouncing or lateral instability, the cardiovascular system must work overtime merely to replace the kinetic energy squandered against the ground.
The Mechanical Springs That Store Free Kinetic Energy
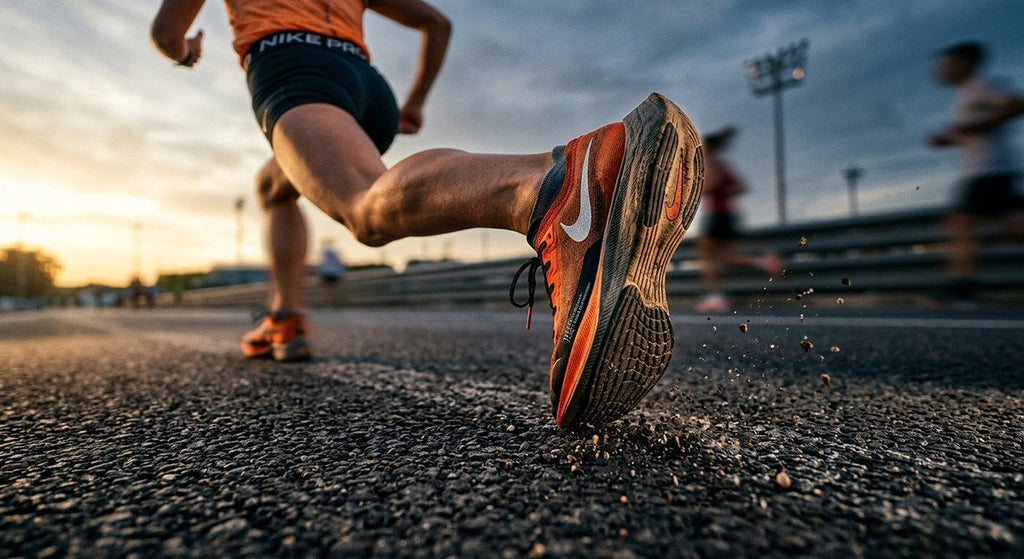
Bipedal running is not a smooth, rolling motion like cycling. It is an alternating chain of single-leg falls, hard collisions, and explosive forward rebounds. When your foot strikes the earth, the skeleton does not simply absorb the blow like an inert block of concrete. Instead, the lower limbs behave like an organic spring-mass system. The Achilles tendon, the plantar fascia under the arch of the foot, and the elastic aponeuroses of the calves stretch under the downward load of body mass, capturing gravitational kinetic energy and storing it as elastic strain energy.
When those connective tissues snap back during toe-off, they release that stored strain energy back into the pavement for free. This mechanical recoil requires zero adenosine triphosphate, the cellular fuel currency driving active muscular contractions. Remarkable findings from Journal of Applied Physiology research on human locomotion demonstrate that tendons can return more than ninety percent of their stored elastic energy during rapid stretch-shortening cycles. Elite distance runners do not necessarily possess bigger quadriceps or larger hearts than their competitors. Instead, they operate with exceptionally stiff, resilient biological springs that propel them down the course without excessive muscular effort.
When an athlete lacks adequate tendon stiffness, the surrounding muscle bellies must contract actively to stabilize each joint upon impact. Active muscular contraction is metabolically costly, whereas passive elastic recoil is metabolically silent. Furthermore, any excessive vertical oscillation, meaning bouncing up and down instead of moving horizontally, sends valuable elastic recoil upward where it does nothing to propel you forward. If a runner bounces just one extra centimeter on every stride over a forty-thousand-stride race, they effectively hoist their entire body weight four hundred vertical meters into the air for zero forward gain.
The Cellular Powerhouses That Conserve Glycogen
Beneath the visible mechanics of posture and stride cadence lies a microscopic world of cellular bioenergetics. Muscle tissue is an intricate mosaic of slow-twitch oxidative fibers and fast-twitch glycolytic fibers wired to separate metabolic pathways. The density of your cellular mitochondria, the specialized organelles that process oxygen, fat, and carbohydrates into muscular work, plays a massive role in elevating running economy without demanding an expansion of overall lung capacity.
When an athlete develops dense mitochondrial networks alongside extensive capillary beds wrapping around individual muscle fibers, oxygen diffusion distances shrink dramatically. Working muscles extract oxygen from circulating blood without forcing the heart to beat at maximum stroke rates. The cardiovascular pump operates under far less strain at any given submaximal cruising pace.
Cellular architecture directly dictates fuel selection. The human body carries tens of thousands of calories in adipose tissue but holds only a small reserve of carbohydrate fuel stored as muscle and liver glycogen. When cellular machinery processes fatty acids efficiently at higher running velocities, the body spares precious carbohydrate stores for the final surge. Preserving glycogen protects neuromuscular junctions from premature fatigue, ensuring strides remain technically sound across the entire duration of an athletic effort.
How Fatigue Silently Destroys Neuromuscular Symmetry
Muscles never act in isolation. The central nervous system acts as an orchestral conductor, regulating the firing rate, motor unit synchronization, and timing of hundreds of muscles simultaneously. In an unconditioned athlete, opposing muscle groups frequently fight one another. When the quadriceps fire to extend the knee, the hamstrings may fail to relax completely, producing antagonist co-contraction. This internal braking action forces the body to burn metabolic energy simply to overcome its own muscular resistance.
Fatigue magnifies these movement flaws rapidly. As core stabilizers and hip abductors tire, pelvises drop, knees cave inward, and forward torso angles collapse. These unforced biomechanical errors that degrade running economy long before cardiovascular fatigue sets in force the body to absorb punishing braking forces with every ground contact.
This cascading mechanical breakdown mirrors systemic risk patterns across other complex disciplines. Just as early negative market swings permanently damage a retirement portfolio before capital can recover, a dynamic explored thoroughly in Sequence of Returns Risk and 4 Proven Defenses That Protect Lifetime Wealth, a runner who burns through structural reserves early in an event triggers compounding mechanical degradation down the stretch. Once movement form breaks down, the oxygen cost of holding a target velocity escalates drastically, turning a smooth aerobic cruise into an exhausting struggle for survival.
Four Proven Pillars That Sharpen Locomotor Output
Building superior movement efficiency does not happen by accident, nor does it develop by simply piling on mindless junk mileage at an unvaried cruising speed. It requires focused structural and neuromuscular adaptations designed to transform the lower limbs into elastic springs.
Heavy Resistance Work for Maximum Motor Unit Recruitment
Endurance training folklore long perpetuated the myth that heavy weightlifting makes runners bulky, heavy, and slow. Modern exercise physiology has thoroughly dismantled that misconception. Lifting heavy loads, specifically three to six repetitions using foundational compound movements like back squats, Romanian deadlifts, and heavy step-ups, triggers neurological adaptations without producing unwanted muscle bulk. Heavy strength training teaches the central nervous system to recruit high-threshold motor units rapidly and coordinate muscular contractions. When the brain can call upon a larger pool of muscle fibers, it rotates through those motor units sequentially during endurance locomotion, delaying local muscular exhaustion and keeping mechanics sound.
Plyometric Loading for Greater Tendon Recoil
If tendons function as biological rubber bands, plyometrics represent the training tool that tunes their recoil capacity. Controlled jumps, ankle pogo hops, bounding drills, and box drops train the lower leg complex to absorb rapid eccentric loads and instantly transfer that force into a snappy concentric rebound. This directly transforms your running economy by teaching connective tissues to return kinetic energy rather than dissipating it as heat. Consistent plyometric work increases collagen cross-linking and elevates tendon stiffness. A stiffer Achilles tendon does not restrict range of motion. Instead, it creates an explosive spring that snaps off the ground in milliseconds, shortening ground contact time and saving muscular energy.
Stride Cadence Optimization to Cut Braking Forces
Overstriding remains one of the most widespread mechanical flaws across the running community. Landing with the foot placed far ahead of the center of mass turns the leg into an emergency brake, sending harsh shockwaves up the shin while violently slowing forward momentum. Increasing step frequency by five to eight percent naturally shifts the landing point directly beneath the pelvis. Stride cadence optimization remains one of the most reliable levers for improving running economy across all skill tiers. A compact, rhythmic cadence cushions ground impact forces, curbs braking decelerations, and utilizes natural elastic rebound to carry the runner forward with minimal muscular strain.
Submaximal Aerobic Volume for Capillary Architecture
Patience remains the rarest virtue in endurance development. Too many athletes spend their training weeks stuck in a moderate-intensity rut, running too hard on easy days and showing up exhausted on hard days. True cellular efficiency requires substantial volume performed at strictly submaximal intensities, well below the first ventilatory threshold where conversational breathing is effortless. Low-intensity volume stimulates vascular endothelial growth factor, signaling the vascular network to construct extensive capillary beds around slow-twitch muscle fibers. It also accelerates mitochondrial biogenesis. These cellular structures cannot be forced through high-intensity intervals alone; they require cumulative hours of easy, conversational training to establish the metabolic foundation that supports speed.
Methods for Monitoring True Locomotor Efficiency
Tracking meaningful progress does not demand regular access to an Olympic laboratory equipped with metabolic gas hoods. While laboratory testing provides exact milliliters of oxygen consumed per kilogram of body weight, several reliable field indicators show whether your mechanics are growing more frugal.
One valuable indicator is the decoupling between heart rate and running pace over prolonged workouts. In an inefficient athlete, holding an identical submaximal speed across flat terrain leads to a steady upward drift in heart rate over seventy to ninety minutes, a phenomenon called cardiac drift. As structural durability, capillarization, and tendon stiffness improve, heart rate stabilizes into a steady plateau across extended distances.
Tracking subtle shifts in running economy across an entire training cycle requires observing heart rate decoupling alongside your rating of perceived exertion. When a running velocity that once felt laboured begins to feel smooth, conversational, and effortless, the body has learned how to glide rather than muscle its way forward. By combining heavy resistance work, plyometric loading, optimized stride cadence, and patient submaximal aerobic volume, you transform your stride from an expensive energy sink into a dynamic, self-propelling kinetic cycle.